
A small repository of the basics to connect the dots.

Extreme environments on Earth
Microbes occupy nearly every niche on Earth. Bacteria and archaea number about 10³⁰ cells, and as many as 3 × 10²⁹ of them live in the marine subsurface, kilometers below the seafloor. Their limits define the physical and chemical boundaries of habitability. Methanopyrus kandleri grows at 122°C at hydrothermal vents, Planococcus halocryophilus divides at −15°C in permafrost brine, and Picrophilus thrives near pH 0. Halophiles grow in salt-saturated brines down to a water activity of about 0.63, the lowest known for any cell. In these settings, life depends on minerals. Where sunlight and organic carbon are scarce, microbes extract energy from rock, oxidizing reduced iron, sulfur and hydrogen released by water–rock reactions. Iron minerals catalyze reactions that microbes perform enzymatically elsewhere, and on the early Earth they probably did so before enzymes existed. Extreme environments are also windows onto other worlds. Hypersaline lakes and evaporite flats resemble the brines and salt deposits on Mars. Perennially ice-covered Antarctic lakes approximate the oceans beneath the ice shells of Europa and Enceladus. Measuring how microbes survive, metabolize and leave biosignatures in these analogues tells us where, and how, to search for life beyond Earth.
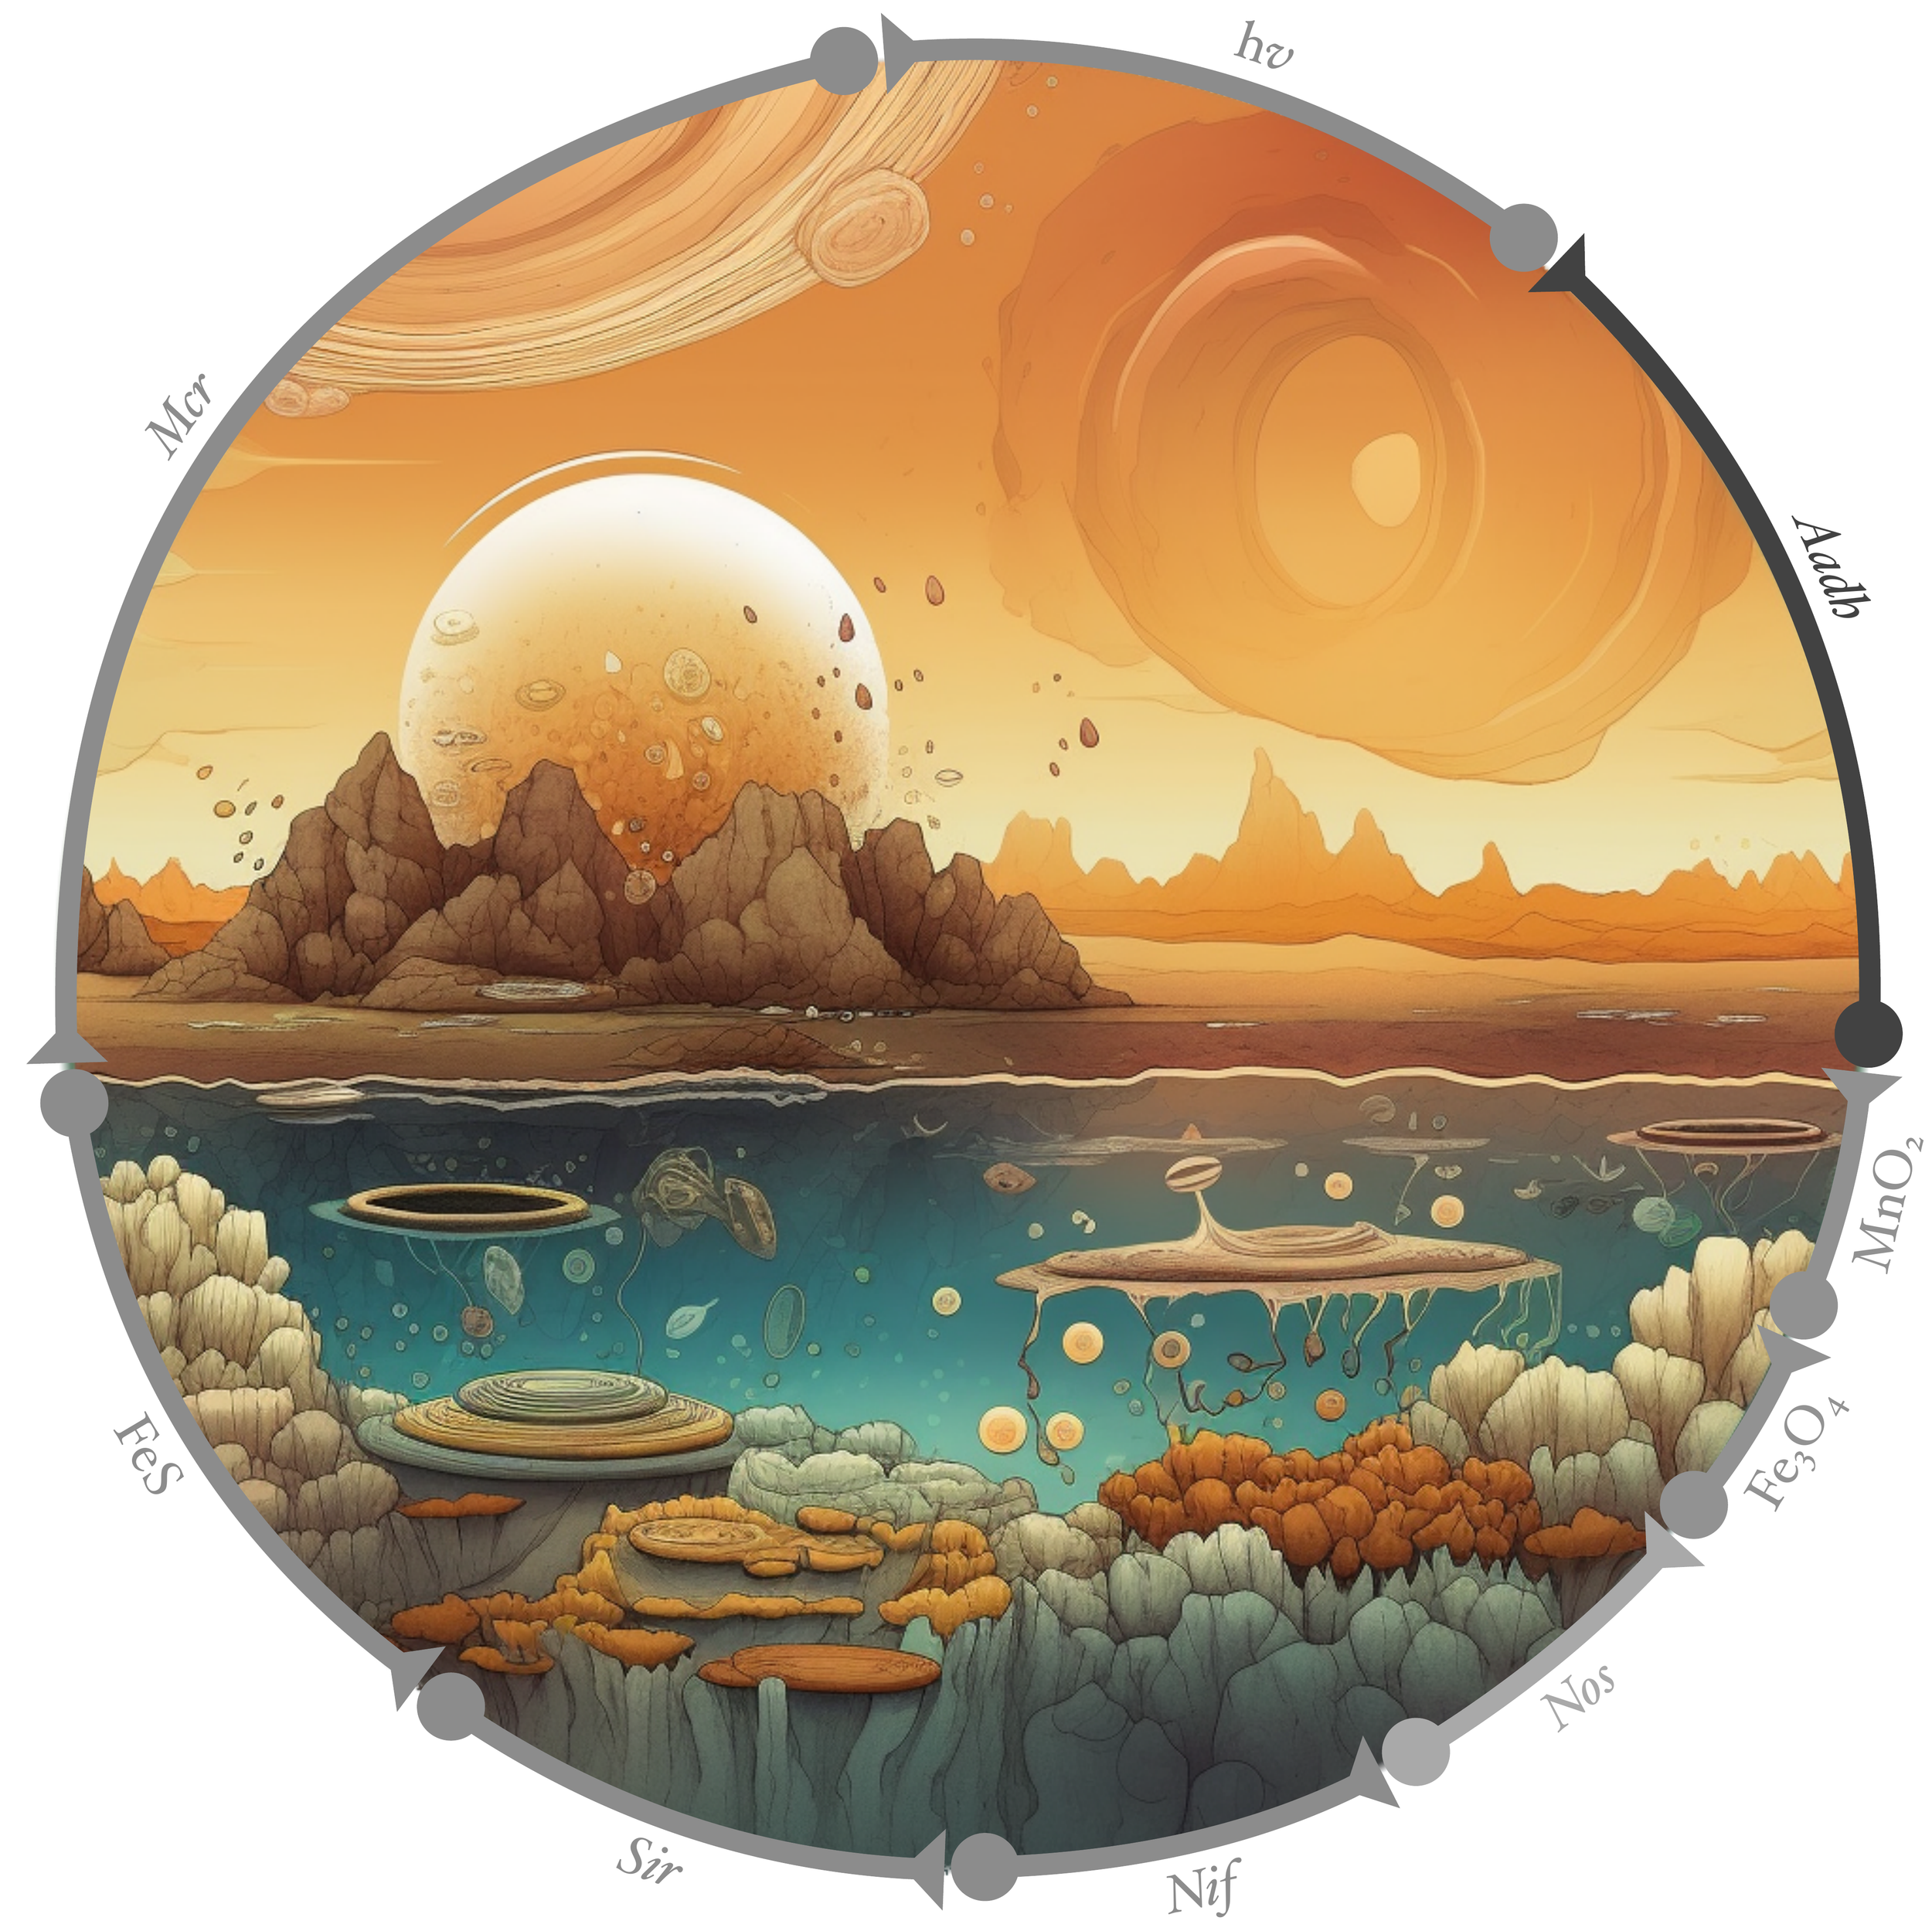
The Gaia hypothesis
In the 1960s, James Lovelock was asked by NASA how to detect life on Mars. His answer was to look at the atmosphere. On a lifeless planet, gases settle toward chemical equilibrium, as on Mars and Venus, where carbon dioxide dominates. Earth's air is far from equilibrium: oxygen and methane coexist although they react with each other, and only constant production by organisms keeps both present. From this observation Lovelock proposed that life does not merely adapt to its planet but regulates it, and he named the idea Gaia.
The evidence is striking. The Sun has brightened by about 30% since life emerged, yet liquid water has persisted for nearly four billion years. Oxygen has stayed within a range that permits both forests and fire for roughly 400 million years. Lovelock's model "Daisyworld" showed how this can work without foresight: dark and light daisies, each growing best at a certain temperature, warm or cool their planet until its temperature stabilizes across a wide range of solar input.
Evolutionary biologists raised a sharp objection. Natural selection favors individuals that leave more offspring, not traits that benefit the planet. A microbe that spends energy cooling Earth would be outcompeted by a "cheater" that enjoys the cooler climate without paying the cost. The answer lies in byproducts. Organisms release oxygen, methane or sulfur gases because doing so serves their own metabolism, and the global effect comes for free. Regulation then arises when these byproducts feed back on growth, and when nutrient recycling closes the loop, so that the waste of one organism becomes the food of another. Species come and go, but the chemical cycles they run persist, because many unrelated organisms can perform the same reaction.
Over geological time, this produces a selection for stability rather than for purpose. Feedbacks that destabilize the environment tend to collapse, whereas stabilizing ones persist and accumulate. Earth's history also records great revolutions, such as the rise of oxygen and the spread of complex cells, in which life tipped the planet into new states and then evolved new regulation. In this view, Gaia is not a designed thermostat but the outcome of life and planet evolving together.

Microcosms
Microcosms bring a piece of the environment into the laboratory. A sample of sediment, water, ice or rock is sealed in a vessel, often a glass bottle capped with a gas-tight butyl rubber stopper, and incubated under defined temperature, salinity, pH and redox conditions. Because the system is closed, every gas produced or consumed accumulates in the headspace, where it can be measured over hours to months. Adding isotopically labeled substrates, such as ¹⁵N-nitrite or ¹³C-bicarbonate, traces individual atoms through metabolic pathways and separates microbial rates from abiotic ones.
The approach dates to the 1880s, when Sergei Winogradsky packed mud into glass columns and watched microbial communities stratify by light, oxygen and sulfide. Modern microcosms pair the same logic with genomics. By changing one variable at a time, they reveal which organisms respond, which genes they express, and how fast they transform carbon, nitrogen, sulfur and iron. Sterile and mineral-only controls distinguish biology from chemistry, a distinction that becomes critical when the question is whether a gas on another planet signals life.

Biosignatures
A biosignature is any substance or pattern whose origin requires life: a fossil cell, an organic molecule, an isotopic fractionation, or a gas that cannot persist without a living source.
Mars once had lakes. Curiosity found organic molecules in 3-billion-year-old mudstones in Gale crater, and Perseverance is sampling an ancient river delta in Jezero crater. Beneath the ice of Enceladus lies an ocean; Cassini flew through its plumes and detected salts, organics, hydrogen and phosphate.
Beyond the Solar System, more than 6,000 exoplanets are known, and the James Webb Space Telescope can now probe their atmospheres. Biosignature gases fall into three classes by how life makes them: waste from energy metabolism (methane, nitrous oxide), byproducts of biomass growth (oxygen), and specialized metabolites (dimethyl sulfide, isoprene, phosphine). The last group is scarce but has few geological sources, making it harder to explain away. Yet nearly every candidate gas can also form without life. Oxygen accumulates from water photolysis, and nitrous oxide forms on iron minerals in anoxic oceans. Distinguishing biological from geological sources will decide whether a detection is a discovery or a false alarm.